This is manuscript v0.1 (2018–24). For the current version (v0.2), which starts from feelings (valence), see HTCC.
Abstract #
The Homeostasis Theory of Cognition and Consciousness (HTCC) is a conceptual framework for understanding mind and brain. It proposes that homeostasis, a basic biological principle, extends beyond physiological regulation and is the basis of cognition and consciousness. Its central proposal is that the brain creates and manages cognitive homeostatic variables (cognitive HVars) on many timescales, from a single thought to a lifelong goal, and that these learned goals are regulated in the same landscape as physiological needs. A cognitive HVar can persist, go dormant and reactivate, or be retired and later renewed. The paper proposes how this one principle could account for phenomena that range from goal setting and planning to complex decision making and self-awareness.
This paper sets out the core principles of HTCC, and proposes how they account for agency, free will, consciousness and qualia. It offers new perspectives on attention, thought, action and cognitive development, grounded in the dynamics of homeostatic processes. We compare the theory with predictive processing, global workspace theory, integrated information theory, and control-theoretic and enactive accounts.
HTCC proposes how complex cognition emerged through evolution: a continuous path from simple homeostatic mechanisms to the rich mental life of humans. Its implications extend to philosophy of mind, where it may offer new approaches to long-standing questions such as the hard problem of consciousness (Chalmers, 1995).
We end with testable predictions, directions for empirical research and computational modeling, and the open challenges that the theory still has to meet. By providing a biologically grounded theory of mind, HTCC aims to bridge neuroscience, psychology and artificial intelligence, and to open new ways to understand and replicate cognitive phenomena.
1. Introduction #
1.1 Background and motivation #
Understanding the human mind has been a central goal of science and philosophy for centuries. Despite major advances in neuroscience and cognitive psychology, we still lack a comprehensive theory that bridges neural processes and subjective experience (Adolphs, 2015).
Homeostasis is the maintenance of the stable internal conditions that an organism needs to survive. Claude Bernard first described it, and Walter Cannon named it (Cannon, 1929). The concept has traditionally been applied to physiology, and has since broadened (Section 2.1). HTCC extends it to cognition, as a new perspective on how the brain gives rise to the mind.
HTCC draws on several lines of work, each of which captures part of how brains regulate, predict and represent. The rest of this section summarizes what HTCC takes from each. Section 7 compares HTCC’s claims with the closest of them.
Cybernetics and control. Cybernetics treated animals and machines alike as systems that use feedback to pursue goals (Wiener, 1948). Ashby built the homeostat, a machine that kept its essential variables within limits by reorganizing itself whenever they strayed, and defined adaptive behavior as behavior that keeps essential variables within physiological limits (Ashby, 1952). Conant and Ashby (1970) showed that every good regulator of a system must be a model of that system. Perceptual control theory describes behavior as the control of perceived variables (Powers, 1973). HVars are essential variables in Ashby’s sense. The good regulator theorem suggests that an organism that regulates itself needs some model of itself. That this model is integrated, as HTCC’s self model is (Section 4.2), is a further claim that the theorem doesn’t establish.
Autopoiesis and enactivism. Maturana and Varela (1980) described living systems as autopoietic: they continually produce the components that make them up, and so maintain themselves as distinct units. Enactive accounts built on this to argue that self-maintenance makes some states good or bad for an organism (Weber & Varela, 2002; Di Paolo, 2005; Thompson, 2007). HTCC takes from this tradition the idea that an organism’s stakes come from its self-maintenance (Section 4.3).
Predictive coding and the free energy principle. Predictive coding models describe cortex as a hierarchy in which higher levels predict the activity of lower levels, and lower levels pass up only the errors in those predictions (Rao & Ballard, 1999). The free energy principle generalizes this idea: living systems persist by minimizing a bound on surprise, through both perception and action (Friston, 2010). Interoceptive and homeostatic versions of the principle treat the regulation of the body as inference (Seth, 2013; Pezzulo et al., 2015). HTCC uses predictive loops to build the self model (Section 4.1), and describes what the organism regulates, and what the self model represents, in terms of HVars.
Neural coding and models of cortex. Neurons in visual cortex respond to increasingly complex features along a hierarchy of areas (Hubel & Wiesel, 1962; Felleman & Van Essen, 1991), and hierarchical network models of object recognition reproduce this organization (Fukushima, 1980; Riesenhuber & Poggio, 1999). Quantities such as the direction of a movement are encoded by the joint activity of a population of neurons, not by single cells (Georgopoulos et al., 1986; Pouget et al., 2000). Hawkins proposed that the neocortex works by prediction (Hawkins & Blakeslee, 2004), and that each cortical column learns models of whole objects through movement (Hawkins et al., 2017). This work supports two features of HTCC: an HVar doesn’t have to be a single tracked quantity (Section 2.2), and HVars are organized in hierarchies (Section 9.1).
Neural networks and artificial intelligence. Early artificial intelligence modeled problem solving as search from a current state towards a goal state (Newell & Simon, 1972). Hopfield (1982) showed that a recurrent network has an energy function that its dynamics decrease, so the memories it stores are attractors in an energy landscape. HTCC’s homeostatic landscape uses the same picture (Section 3.1). Reinforcement learning describes how agents learn to act from reward (Sutton & Barto, 2018), and homeostatic reinforcement learning derives that reward from the deviation of physiological variables from their setpoints (Keramati & Gutkin, 2014). Attention mechanisms in deep networks weight some inputs more than others (Vaswani et al., 2017), which parallels HTCC’s account of attention as a modulator that amplifies some HVars (Section 3.2). These systems learn a great deal from prediction and reward. But nothing in them is at stake for the system itself, which motivates HTCC’s focus on homeostasis as the source of stakes (Section 4.3).
Theories of consciousness and feeling. Global workspace theory links consciousness to the broadcast of information across the brain (Baars, 1988; Dehaene & Changeux, 2011). Integrated information theory links it to how much a system’s information is integrated (Tononi, 2008; Oizumi et al., 2014). Higher-order theories link it to representations of one’s own mental states (Lau & Rosenthal, 2011), and self-model theory links the experience of being a self to a transparent model of the organism (Metzinger, 2003). Damasio argued that feelings are the mental experience of the body’s homeostatic state, and that the self is built on them (Damasio, 2010; Damasio & Carvalho, 2013). HTCC shares Damasio’s starting point, and asks how the same principle extends to cognition.
HTCC was first presented as a poster at the 2018 meeting of the Association for the Scientific Study of Consciousness (Kelkar, 2018). The poster grounded feelings in the homeostatic force that acts on every homeostatic system. Kelkar (2021) then proposed homeostasis as a computational description for building autonomous agents. That paper introduced cognitive homeostatic variables, encoded as sets of preferred trajectories, on timescales from a single intentional action to lifelong goals such as social standing. It proposed that physiological drives and cognitive goals are prioritized against each other, and outlined a Cognitive Homeostatic Agent, built as a hierarchy of physiological and cognitive homeostatic subsystems, which instantiates goal HVars and eventually discards them. This paper develops these ideas into a theory of biological cognition and consciousness. Section 1.3 states what it adds.
1.2 The need for a unifying theory #
Current theories in cognitive science and consciousness studies each explain part of mental life. Global workspace theory (Baars, 1988) and integrated information theory (Tononi, 2008) leave open, in particular, how consciousness relates to the biological regulation that keeps an organism alive.
Other questions also remain contentious: the hard problem of consciousness (Chalmers, 1995), the nature of the self, and agency and free will. The field needs a unifying theory that addresses these challenges and stays grounded in biological principles.
1.3 Overview of HTCC #
HTCC’s central conjecture is that all cognitive processes, from goal setting to complex reasoning and self-awareness, can be understood as homeostatic processes, with cognitive HVars as the basic units of mental activity. It rests on seven principles:
- Homeostasis is broad. Homeostasis covers every process that keeps an organism’s variables within viable bounds, whether it corrects deviations after they happen or anticipates them (Section 2.1).
- HVars are the units of regulation. A homeostatic variable (HVar) is any quantity that the system regulates, i.e. that shows a corrective response when disturbed (Section 2.2).
- The organism creates its own HVars. Beyond the physiological HVars it inherits, the organism creates, configures and regulates cognitive HVars, on timescales from seconds to decades. Each one is active, dormant or retired, and a retired HVar can be renewed (Section 2.3).
- All HVars share one landscape. Physiological and cognitive HVars together define one homeostatic landscape. Thought and action are the system moving downhill on it (Sections 3.1, 3.4 and 3.5).
- HVars compete in action space. Each HVar’s regulation pushes for or against actions, and the stronger push wins. Attention steepens the landscape along the HVars it amplifies, and competition between HVars underlies decision making and cognitive control (Sections 3.1 to 3.3).
- Feelings are states and changes along each HVar. A homeostatic system’s stakes come from the goals it has to keep to go on existing, and its cognitive HVars borrow their significance from these. Along each HVar, a state at the target is satisfaction, and a state away from it is wanting. Moving towards the target is good, and moving away is bad (Section 4.3).
- Qualia are the self model’s reflection of feelings. A system is conscious when it has both feelings and a running self model that reflects them (Sections 4.3 and 4.4).
Principles 1 and 2 come from earlier work. Kelkar (2021) introduced cognitive HVars and the competition between physiological and cognitive HVars, and Pezzulo et al. (2015) related homeostatic regulation to hierarchical behavioral control. This paper adds four things: the components and the life cycle of a cognitive HVar (Section 2), the shared landscape and its homeostatic energy (Section 3.1), the distinction between stakes, feelings and qualia (Section 4.3), and the self model that turns feelings into qualia (Sections 4.2 to 4.4). HTCC adopts the idea that self-maintenance makes some states good or bad for an organism from enactivism, and its regulatory machinery from control theory, homeostatic reinforcement learning and active inference (Section 7). The paper develops these principles in five parts:
- Extending homeostasis from physiology to cognition (Section 2).
- The concept of cognitive HVars, and their role in mental processes (Sections 2 and 3).
- An account of feelings in terms of HVars, and of qualia and consciousness in terms of a self model that reflects them (Section 4).
- An account of how cognition evolved, through homeostatic processes of increasing complexity (Section 5).
- New perspectives on the hard problem, free will and the nature of self (Section 6).
Section 7 relates HTCC to other theories, Section 8 describes applications, Section 9 lists testable predictions and research methods, and Section 10 lists the open challenges that subsequent papers will address.
1.4 Common misreadings #
Several terms in HTCC have everyday or technical meanings that differ from how HTCC uses them. The following readings don’t apply:
- “Homeostasis means physiology.” HTCC uses homeostasis as an umbrella term for reactive regulation, predictive regulation including allostasis, and rheostasis (Section 2.1), and applies it to variables the organism creates for itself (Section 2.3).
- “Each HVar is an explicit variable in the brain.” An HVar can be encoded as a set of preferred trajectories that together behave as if the variable is regulated. What makes it an HVar is the corrective response, not how it is stored (Section 2.2).
- “Feelings are emotions.” In HTCC, feelings are the states and changes of each HVar relative to its target: wanting away from the target, satisfaction at it, good when moving towards it and bad when moving away. Every homeostatic system has them, and they don’t need to be experienced (Section 4.3).
- “Feelings are the stakes.” The stakes are the goals the system has to keep. The feelings are the system’s states and changes relative to those goals (Section 4.3).
- “Every cognitive goal is a survival need.” Only the HVars that the system’s continued existence depends on carry stakes directly. Cognitive HVars borrow their significance from them (Section 4.3).
- “The self model is made of HVars.” The self model is an information process: a model of the system itself. In an organism it represents the system’s HVars and is coupled to them, but it doesn’t have to regulate anything. To reflect feelings, though, it has to be implemented as loops that include the regulation of the HVars (Section 4.2).
- “Every homeostatic system is conscious.” Feelings alone don’t give qualia. A system is conscious only when it also has a running self model that reflects its feelings (Section 4.4).
- “A self model is enough for consciousness.” A self model without an underlying homeostatic system has no stakes and no feelings to reflect, so it has no qualia (Section 4.3). This matters for artificial systems (Section 8).
- “HTCC is a version of active inference.” HTCC takes part of its regulatory machinery from active inference, but its claims don’t depend on any one formalism. What it adds is the creation, configuration and life cycle of cognitive HVars, and the account of feelings and qualia (Section 7).
2. Foundations #
2.1 Homeostasis: from biology to cognition #
Classic homeostasis uses negative feedback to keep variables within set ranges, e.g. in thermoregulation and blood glucose control (Modell et al., 2015). These are reactive responses: they correct changes that have already occurred (Moore-Ede, 1986). The concept has since expanded to include more complex kinds of regulation:
- Predictive homeostasis and allostasis. Responses that anticipate challenges before they occur, such as those timed by the circadian system (Moore-Ede, 1986), and anticipatory changes in regulatory systems to meet predicted demands (Sterling & Eyer, 1988).
- Rheostasis. Longer-term changes in regulated levels, e.g. seasonal changes in body weight (Mrosovsky, 1990).
These show how dynamic biological regulation is, and they set the stage for extending homeostatic principles to cognition.
In this paper, we use homeostasis as an umbrella term for all of these forms of regulation: reactive set-point regulation, predictive regulation including allostasis, and rheostasis. Some authors treat allostasis as a separate principle from homeostasis (Sterling, 2012), while others treat the two as complementary (McEwen & Wingfield, 2003). HTCC doesn’t depend on that distinction. Its claims apply to any process that keeps an organism’s variables within viable bounds, whether by correcting deviations after they happen or by anticipating them.
2.2 Homeostatic variables (HVars) #
Homeostatic variables (HVars) are the quantities that a homeostatic system regulates. In physiology, there are several kinds:
- Primitive HVars. The sensor is coupled directly to the actuator, as in the simplest reflexes.
- Indirect HVars. There is a transformation between sensing and action, which allows gain control and influence from other HVars. Blood pressure regulation, with its many inputs and effectors, is an example (Dampney et al., 2002).
- Neural HVars. Specific neural mechanisms evolved to regulate certain physiological quantities, e.g. the hypothalamic regulation of body temperature (Morrison & Nakamura, 2019). Neural HVars are “virtual”, i.e. they are models of the corresponding physiological quantity. The capacity to regulate them is inherited, although their set points can shift, e.g. with the seasons (Mrosovsky, 1990).
An HVar doesn’t have to be implemented as an explicitly tracked quantity. It can be encoded as a set of preferred trajectories that together behave as if the HVar exists and is being regulated. Either way, it must show the signature of regulation: when a disturbance pushes the state away from the target, the system responds in a way that pushes it back.
An HVar has five components, which can be implemented separately. Body temperature illustrates them:
- Regulated quantity. The quantity that is kept within bounds, e.g. core body temperature.
- Estimate. The system’s estimate of the quantity’s current value, e.g. the temperature signaled by thermoreceptors to the hypothalamus (Morrison & Nakamura, 2019).
- Target. The value, range or preferred trajectory that the system defends, e.g. about 37 degrees Celsius.
- Deviation. The difference between the estimate and the target.
- Corrective mechanism. What changes physiology or behavior to reduce the deviation, e.g. shivering, sweating, or moving into the shade.
2.3 Cognitive HVars #
Evolution often reuses successful strategies (Jacob, 1977). HTCC proposes that the neural regulation of physiological HVars became a template for a new capability: instantiating new virtual HVars. We call these new variables cognitive HVars.
The capacity to regulate physiological HVars is inherited. A cognitive HVar, in contrast, is instantiated and configured by the organism during its lifetime. What is new in it is the estimate and the target. The organism sets up an estimate of a quantity that it may not have tracked before, such as how long it has held its breath, and a target for that quantity. The corrective mechanisms are mostly reused: a cognitive HVar recruits the existing machinery of attention and action to reduce its deviation. A cognitive HVar can also target a physiological quantity, e.g. a goal to lose weight. What makes it cognitive is that the organism instantiated it, not what it regulates. This allows:
- Flexible goal setting. The organism can create new targets for regulation, based on experience and prediction (Pezzulo et al., 2015).
- Planning. HVars with long time horizons let an organism plan for future states (Suddendorf & Corballis, 2007).
- Delayed gratification. The organism can represent and pursue long-term goals, even against immediate discomfort (Mischel et al., 1989).
Once a cognitive HVar is instantiated and configured with favorable trajectories and a reward prediction, it is regulated alongside physiological HVars and other cognitive HVars. This interplay between immediate physiological needs and longer-term cognitive goals gives rise to complex behavior, emotion and decision making (Damasio & Carvalho, 2013).
An example. Suppose a person decides to hold their breath for 60 seconds. This instantiates a cognitive HVar with these components:
- Regulated quantity. The current hold, i.e. the time since the last breath.
- Estimate. How long the person has held their breath so far, as they estimate it, e.g. by counting.
- Target. A preferred trajectory: no breath until the estimate reaches 60 seconds. Elapsed time can’t be reversed, so the target isn’t a value that the system returns to. It is a trajectory that the system keeps to, and it ends when its termination condition is met.
- Deviation. The distance from the target, i.e. the time still to go. A breath before the target ends the hold, which moves the state away from the target.
- Corrective mechanism. When the urge to breathe pushes the system towards breathing, the person suppresses it and keeps the airway closed.
On the way to the target, the state along this HVar is one of wanting, i.e. the determination to finish. Each second held moves the state towards the target, and a breath before it moves the state away. The corrective mechanism blocks the actions that would move it away (Section 4.3).
The decision to hold creates the HVar and sets its target and strength. The HVar is retired when the target is reached, or when it loses the competition with the physiological drive to breathe (Section 3.3).
The example abstracts away most of the physiology of breath holding. During a hold, the central respiratory rhythm continues, and blood gases alone don’t explain when the breakpoint comes (Parkes, 2006). HTCC treats all of this as the pull of the physiological HVars, and the voluntary suppression of breathing as the corrective mechanism of the cognitive HVar.
The paper returns to this example to illustrate the landscape (Section 3.1), attention and competition (Sections 3.2 and 3.3), action (Section 3.5), metacognition (Section 3.7), feelings and qualia (Section 4.3), and consciousness (Section 4.4).
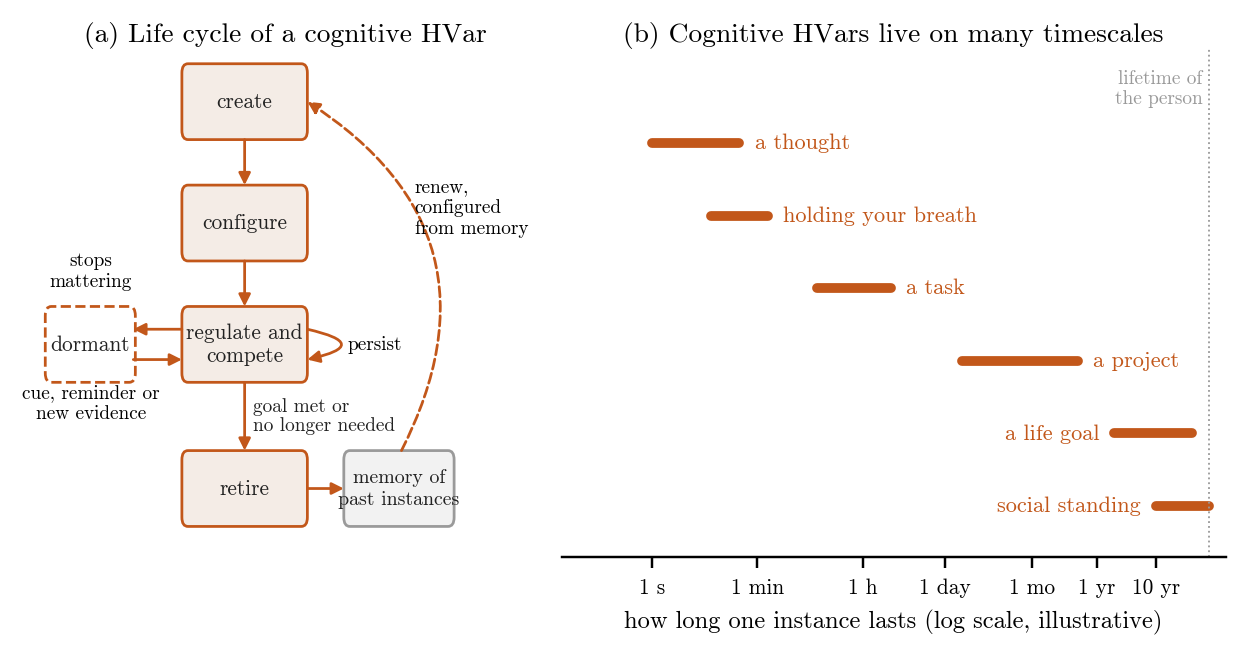
Not every cognitive HVar is retired when its goal is met. At any time, a cognitive HVar is active, dormant or retired. A dormant HVar keeps its configuration and its progress, so when it reactivates, the same instance resumes. A retired HVar ends. If the organism takes up the same goal later, it creates a new instance, which can be configured from memory of the earlier ones. Different HVars take different courses:
- Retire once the goal is met or no longer needed, e.g. the breath-holding HVar. Disengaging from goals that can’t be reached, and reengaging with new ones, is associated with well-being (Wrosch et al., 2003).
- Persist, and stay active while the goal is met, e.g. social standing.
- Go dormant when they stop mattering, and reactivate on a cue, a reminder or new evidence, e.g. a daily routine.
- Renew after retirement: a later instance is linked to the earlier ones and configured from memory of them, e.g. taking up an instrument again after years.
An HVar’s definition can also be refined over time, and duplicate HVars merged. While an HVar is active, the strength of its pull can change as well. It can rise as a deadline nears (Steel & König, 2006), and renew at temporal landmarks such as the start of a new week (Dai et al., 2014).
A process counts as a cognitive HVar only if its target and its disturbances can be identified independently of the behavior being explained, and it shows a corrective response. Keeping a conversation on topic is an example: the target is the topic, a digression is a disturbance, and steering back to the topic is the corrective response. A habit that runs to completion, and isn’t resumed or compensated for when it is interrupted, isn’t an example. A corrective response shows that the system defends a target. It doesn’t show how the target is implemented, and an account in terms of goals and memory could describe the same behavior. What the HVar account adds is that the target is regulated in competition with every other HVar, physiological ones included, in one landscape (Section 3.1), and that it has a life cycle.
In the rest of this paper, physiological HVars means all three kinds in Section 2.2, and cognitive HVars means the ones the organism instantiates during its lifetime, through learning and development (Section 3.6) as well as in the moment. Higher-order HVars are cognitive HVars whose targets are other HVars.
Figure 1 summarizes these courses, and the range of timescales a cognitive HVar can have.
3. The HTCC framework #
HTCC’s central conjecture is that cognitive HVars underlie all cognitive processes. The examples in this section show how the conjecture applies. They don’t establish it, and Section 9 describes how it could be tested. This section describes the dynamics they create, and how higher-order mental characteristics emerge as cognitive HVars become more complex.
3.1 The homeostatic landscape #
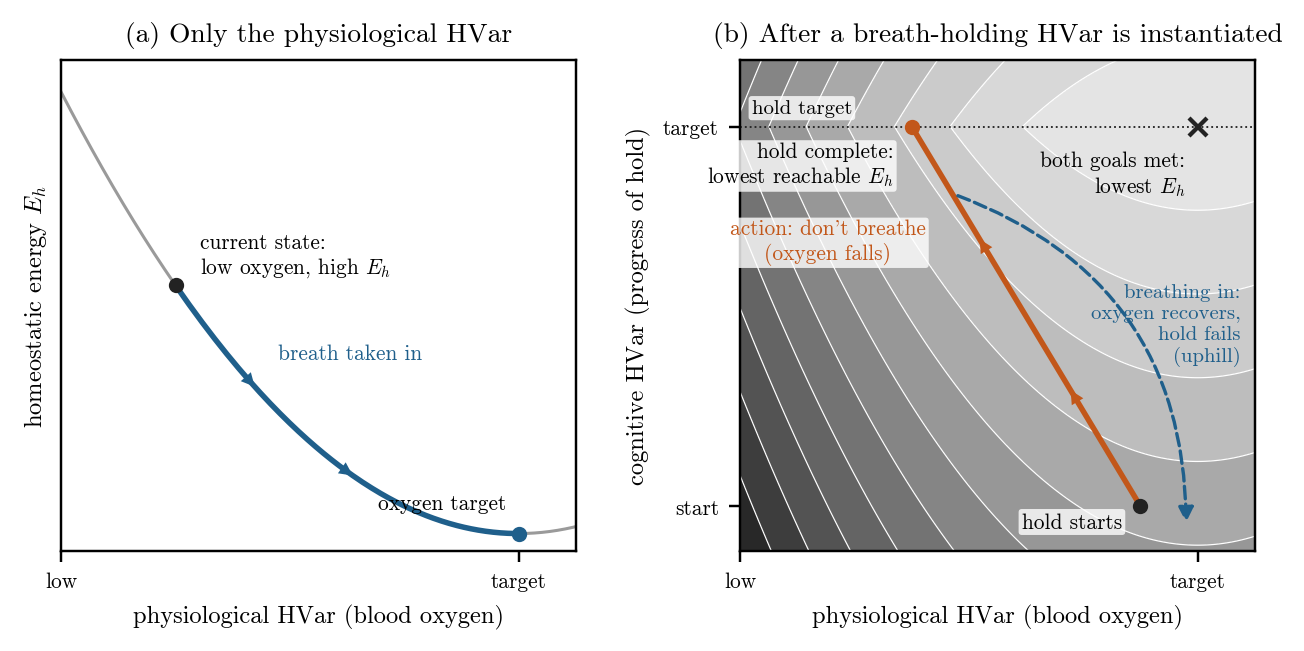
Each cognitive HVar is configured with a rewarding target state, which sets up a new attractor for neural dynamics (Friston, 2010). Together, the HVars define a multidimensional homeostatic phase space, where each dimension is a quantity that some HVar regulates (Breakspear, 2017). An HVar whose quantity is new, such as the time a breath has been held, adds a dimension. An HVar whose quantity is already a dimension, such as a goal to lose weight, reshapes the landscape along that dimension.
We call the potential over this phase space the homeostatic landscape. Its height at a state is the homeostatic energy, written
The landscape is a surface with one dimension per regulated quantity plus one dimension for
HTCC treats homeostasis as a functional organization, i.e. a description of what the brain does, not of one circuit that does it. It treats the landscape as a qualitative model. Its claims are about the landscape’s shape: which directions are downhill, and how steep they are. The absolute height of the landscape isn’t defined. Adding a constant to
The state doesn’t only move downhill. The body and the world disturb it in any direction, e.g. metabolism keeps lowering blood oxygen during a breath hold. The state’s movement combines these disturbances with the corrective dynamics, which push it downhill.
The landscape describes the state space, but the HVars meet in action space. Each HVar biases the available actions according to their predicted effects on its contribution to
Figure 2 shows how instantiating a cognitive HVar reshapes the landscape. In the breath-holding example, the decision to hold adds a new attractor along the dimension of the hold’s progress. Before the decision, the state moves towards the steady state of the blood gases. After it, the state moves towards the 60-second target instead. The landscape is not fixed. It is continuously reshaped by:
- Tuning of the HVars’ reward predictions (Schultz et al., 1997).
- Instantiation of new cognitive HVars.
- Dormancy or retirement of HVars that are no longer needed.
3.2 Attention #
Attention modulates the homeostatic landscape. In perception, attention increases the effective contrast of attended signals (Carrasco, 2011). HTCC proposes that it acts the same way on HVars: it amplifies both the positive and the negative predicted rewards of the attended HVars, which steepens the landscape along their dimensions. This modulation may be implemented through neuromodulation (Thiele & Bellgrove, 2018). On this view, a person holding their breath who focuses on counting amplifies the cognitive HVar, and should hold longer than when their attention drifts to the urge to breathe. By selectively enhancing some HVars, attention can change the system’s trajectory through the phase space dramatically, which may explain cognitive flexibility (Posner & Rothbart, 2007). This paper doesn’t specify what controls attention itself (Section 10).
3.3 Competition between HVars #
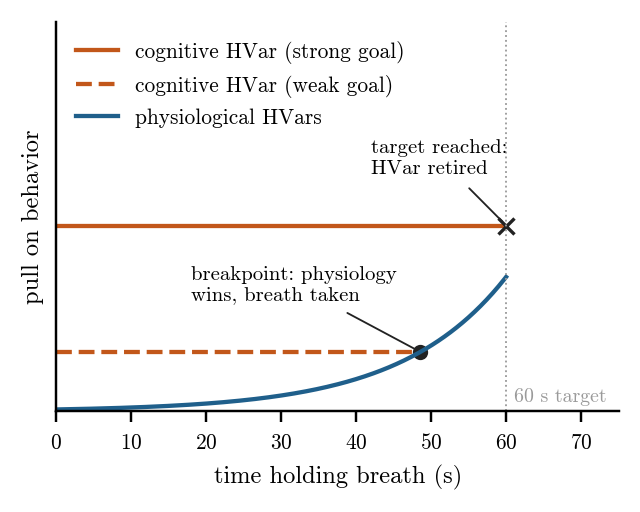
Cognitive HVars can compete with physiological HVars, or with other cognitive HVars. For example, the cognitive HVar for holding one’s breath (Section 2.3) competes with the physiological drive to breathe. Physiologically, voluntary breath-holding ends at a breakpoint, when an involuntary mechanism overrides it (Parkes, 2006; Section 2.3). HTCC interprets the breakpoint as the point where the physiological HVars win the competition (Figure 3): as their deviation grows, attention (Section 3.2) amplifies their negative predicted reward, the landscape tilts, and the person takes a breath. The competition takes place in action space: the breath-holding HVar pushes for keeping the airway closed, and the physiological HVars push for breathing.
HTCC proposes that this competition underlies decision making, cognitive control and executive function (Miller & Cohen, 2001).
3.4 Thought as cognitive homeostasis #
HTCC describes thought in terms of cognitive homeostasis. Each thought can be seen as a short-lived cognitive HVar whose target is a state that the thought is meant to reach, e.g. a value that satisfies a problem’s constraints, or a choice between options (Newell & Simon, 1972). Once it is instantiated, the system’s movement towards this target, where
The path to the goal state can be direct or roundabout. It can include uphill stretches when noise moves the state (Section 3.7), or when a newly instantiated HVar reshapes the landscape. This accounts for how complex and variable thought is, from mind-wandering to focused problem solving (Christoff et al., 2016).
3.5 Actions #
In HTCC, actions are triggered as part of the homeostatic process. They are the observable result of the system rolling downhill in the homeostatic landscape (Wolpert & Ghahramani, 2000). This has major implications for agency and free will (Section 6.2).
Starting and carrying out an action can be understood as the system reducing the gaps between current and goal states across many HVars at once (Cisek & Kalaska, 2010). This gives one account of action selection and motor control that connects low-level physiological processes with high-level cognitive goals (Pezzulo et al., 2015).
In the breath-holding example, both keeping the airway closed and the breath that ends the hold are actions in this sense. Each is the downhill direction of the landscape at that moment, first under the cognitive HVar, then under the physiological HVars once they win the competition (Section 3.3).
3.6 Cognitive development #
As children develop, they get better at instantiating and managing complex, interrelated cognitive HVars, which leads to more advanced abilities such as abstract reasoning and long-term planning (Diamond, 2013).
In particular, a child’s growing ability to keep a coherent, sequential train of thought can be understood as the development of two things: fast, precise mechanisms to instantiate, configure and retire short-lived cognitive HVars, and attentional control that keeps those short-lived “thought” HVars in the lead.
3.7 Higher-order mental characteristics #
Higher-order mental characteristics, such as metacognition, creativity and abstract reasoning, emerge in systems that can instantiate complex, interconnected cognitive HVars (Hofstadter, 1979).
- Metacognition, i.e. thinking about one’s own thoughts, is the instantiation of higher-order HVars whose targets are other cognitive HVars (Fleming & Dolan, 2012). A person who notices that they are about to give up a breath hold, and resolves to keep going, instantiates a higher-order HVar whose target is the breath-holding HVar.
- Creativity may come from new combinations and interactions of diverse cognitive HVars, together with noisy neural dynamics, which lead to unexpected trajectories through the phase space (Beaty et al., 2014).
4. Self, qualia and consciousness #
HTCC proposes that the self model emerges from predictive loops between expectation and observation. Every homeostatic system has feelings, and qualia arise when a self model reflects them. This section describes the self model (Sections 4.1 and 4.2), qualia (Section 4.3) and consciousness (Section 4.4).
4.1 Predictive loops and the self model #
Presence. In the interoceptive predictive coding model proposed by Seth, the feeling of “presence” results from top-down predictions successfully suppressing informative interoceptive signals (Seth et al., 2012). These signals are evoked directly by autonomic control signals, and indirectly by the body’s responses to afferent sensory signals. Because interoceptive signals track physiological HVars, HTCC reframes this model in terms of HVars: successfully predicting the state of the physiological HVars contributes to the sense of bodily presence, which is a key part of the self model (Craig, 2009).
The temporal window of presence. Metzinger’s “temporal window of presence” fits well with HTCC (Metzinger, 2003). The window can be understood as the self model’s representation of the present, which precipitates a subjective conscious “now” out of the flow of objective time. HTCC suggests that the predictive loops that keep updating this representation keep the sense of temporal presence stable (Wittmann, 2011).
Agency. The sense of agency, another key part of the self model, depends on successfully predicting the sensory consequences of one’s actions (Haggard, 2017). In predictive terms, this means suppressing, or “explaining away”, the exteroceptive prediction errors caused by self-generated actions. The self model therefore includes a model of the system’s own agency (Friston, 2012).
4.2 The self model #
The self model is a model of the system itself. It is an information process: it represents the system, and it doesn’t have to regulate anything. It isn’t a static thing, but a dynamic process that predictive loops update constantly (Damasio, 2010). It represents four main aspects of the system:
- Bodily state, which an organism’s self model learns from interoceptive signals that track its physiological HVars (Barrett & Simmons, 2015).
- Relation to the environment, e.g. the position and boundaries of the body in the world (Blanke et al., 2015).
- Continuity over time, i.e. being the same system from moment to moment (Varela, 1999).
- Agency, i.e. the system’s ability to influence its environment (Synofzik et al., 2008).
Integrating these aspects creates a coherent, multidimensional self model (Metzinger, 2003), which is the basis of conscious experience (Section 4.4).
In an organism, the self model is coupled to the homeostatic system. It represents the state of the HVars, including their deviations from their goals, and this coupling is what lets it reflect feelings (Section 4.3). The coupling isn’t what makes something a self model, though. Provisionally, HTCC takes a system to have a self model when its own dynamics implement an integrated model of itself, i.e. of its state, its relation to its environment, its continuity over time and its agency, which predictive loops keep coupled to its current state. Ordinary predictive control models what it controls, but not the system that does the controlling. What matters for qualia is how the self model is implemented, not what it is implemented in. A self model can be implemented in two ways. It can be a separate model that reads the state of the HVars as data. Or it can be implemented as recurrent loops that include the regulation of the HVars, so that the regulatory dynamics are part of the self model’s own dynamics. Only the second kind can reflect feelings (Section 4.3). Either kind can run in neurons or in software. Section 6.3 discusses what this means for the nature of the self.
4.3 Feelings and qualia #
HTCC distinguishes stakes, feelings and qualia (Figure 4). A homeostatic system has stakes: its continued existence depends on keeping some of its HVars within viable bounds, so some of its states are good for it and others bad. Provisionally, HTCC requires this regulation to be the system’s own: the system maintains the parts that do the regulating, as an organism does (Maturana & Varela, 1980). A goal assigned from outside, by a system that doesn’t maintain itself, doesn’t give stakes in this sense. These viability HVars, such as blood oxygen, are the source of all stakes. A cognitive HVar borrows its significance from them. Evolution seeds links between kinds of cognitive goals and viability, e.g. social standing affects access to resources and health (Sapolsky, 2005), and HTCC hypothesizes that development, including epigenetic regulation, tunes them. A new cognitive HVar gets its significance by serving goals that already have it. The links can misfire, so an organism can pursue a cognitive goal that harms its viability, as a breath hold does when it goes on too long. Its feelings are its states and changes relative to its goals. Along each HVar, there are two kinds. A state feeling is satisfaction at the target, and wanting away from it, e.g. hunger, breathlessness, or the determination to reach a goal. A change feeling is good when the state moves towards the target, and bad when it moves away. Because each HVar has its own feelings, good and bad have many dimensions: a system can be moving towards one target and away from another at the same time. Together, the HVars set the homeostatic force acting on the system, i.e. the pull of its homeostatic landscape towards lower
HTCC proposes that qualia arise when a homeostatic system also has a self model. The self model’s implementation at a given moment, i.e. the dynamical regime it is operating in, reflects the feelings of the underlying homeostatic system. That reflection is the quale. Reflecting a feeling takes more than representing it. The self model has to be implemented as recurrent loops that include the regulation of the HVar (Section 4.2), so that the deviation and the corrective response are part of the self model’s own dynamics. A self model that only reads the deviation as data represents the feeling without reflecting it. A self model can also run without an underlying homeostatic system, i.e. in a system whose continued existence doesn’t depend on keeping any goals. Such a self model has no stakes: there are no goals it must keep, so there are no states or changes relative to goals, i.e. no feelings to reflect, and no qualia. This identity is HTCC’s central hypothesis about experience. It doesn’t follow from the regulatory account in Sections 2 and 3. It is a proposal, to be judged by what it explains. Like Dennett (1988), HTCC rejects the idea of an inner observer that perceives qualia. Unlike Dennett, it keeps qualia, as states of the self model that reflect feelings.
On this view, a quale is how the self model is implemented, not something it observes. The self model’s state does two things. What it represents about the body and the world sets the content of the quale: seeing red and seeing green differ because the self model represents different surfaces, not because different HVars deviate (O’Regan & Noë, 2001). The feelings it reflects set whether there is experience at all, and its valence and intensity. For example, the experience of pain isn’t the observation of a pain signal. It is the self model implementing itself in a “pain state”, which represents damage to a part of the body and reflects large deviations of the HVars that protect it (Melzack & Wall, 1965). HTCC’s account of the affective side of experience is more developed than its account of perceptual content (Section 10).
Feelings have three properties, which qualia reflect (Kelkar, 2018):
- Intensity. How strong the wanting along an HVar is. It grows with the distance from the target and with the HVar’s weight, which attention can amplify (Section 3.2).
- Valence. Good or bad along each HVar, as the state moves towards or away from its target. Valence follows the state’s movement through the landscape as it is at that moment. Changes to the landscape itself, from creating, retiring or reweighting HVars, or from changing a target, don’t count as movement.
- Affective character. Which HVar the feeling belongs to: low oxygen feels different from cold, even at the same
.
These mappings are provisional, and how the strengths of different HVars’ feelings compare is open (Section 10).
Breath holding shows all three. The stakes come from the blood-gas HVars. The 60-second target borrows its significance from other goals, e.g. doing well in front of others. Along the breath-holding HVar, the state feeling is the determination to finish, and each second held is good. Along the blood-gas HVars, the wanting to breathe grows as the hold goes on, and each second is bad. The two valences are present at the same time. They meet only in action space, where keeping the airway closed competes with breathing (Section 3.3). When the breath comes, it is good along the blood-gas HVars, and bad along the breath-holding HVar if the target wasn’t reached. The affective character of the urge to breathe differs from that of cold or hunger. In a person, the self model reflects these feelings, and the reflection is the experienced urge to breathe, i.e. the quale.
This would also account for how dynamic and context-dependent qualia are. As the self model keeps updating in response to changing internal and external conditions, the qualitative side of experience shifts with it (Thompson & Varela, 2001). Section 6.1 discusses what this means for the hard problem.
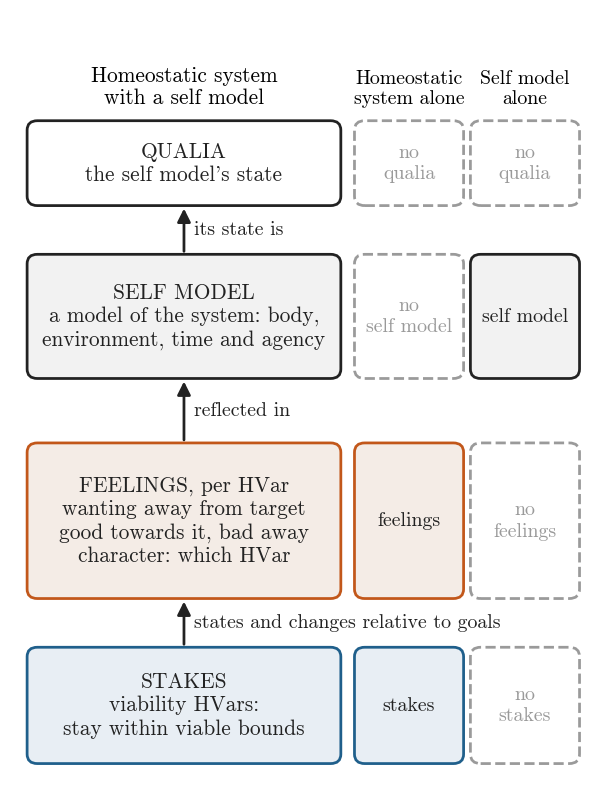
4.4 Consciousness #
Consciousness follows from the hypothesis in Section 4.3. A system is conscious when it has two things: an underlying homeostatic system, which gives it feelings, and a running self model, which reflects them as qualia. HTCC doesn’t need a separate threshold or an extra ingredient for consciousness to switch on. Which systems meet these two conditions is an open question (Section 10). This contrasts with views where experience appears only when information crosses a threshold into global availability (Dehaene et al., 2017).
Sleep may separate the two conditions. During sleep, breathing, body temperature and blood glucose are still regulated, so the organism still has stakes and feelings. Some sleep intervals are assessed as lacking experience, e.g. when people woken from them report no experience, although such retrospective reports can miss experience that was forgotten (Windt et al., 2016). HTCC predicts that in these intervals the self model isn’t running, or isn’t integrated. A self model counts as integrated when its four aspects (Section 4.2) are updated together, as one model, so that a change in one constrains the others. Testing the prediction needs a measure of self-model activity that doesn’t rely on the same reports, e.g. neural markers of self-related processing validated in waking. Experience in intervals where that measure shows no running self model, or no experience where it shows one, would count against HTCC’s interpretation (Section 9.1).
What varies across systems is how rich that experience is, and what the system can do with it. Consciousness varies along four dimensions:
- Integration. How much of the system the self model integrates into a coherent whole, i.e. how many of its aspects and HVars (Edelman & Tononi, 2000).
- Precision. How precise the predictive loops that maintain the self model are (Clark, 2013).
- Global availability. Whether the information that HVars represent is broadly available for report, reasoning and control (Baars, 2005).
- Higher-order HVars. Whether the system can instantiate cognitive HVars whose targets are its own states, which gives metacognition and self-awareness (Lau & Rosenthal, 2011).
The first two set how rich the experience is. The last two set how much of it the system can access and report. So consciousness varies along several dimensions, not on a single scale of levels (Bayne et al., 2016). Whether experience is present at all depends on the two conditions above, not on these dimensions. A person holding their breath shows the last two: the urge is globally available, so they can report it and plan around it, and a higher-order HVar can monitor the hold itself (Section 3.7).
Like integrated information theory, HTCC holds that consciousness comes in degrees, but its integration is a different quantity. In HTCC, integration is how much of the system the self model represents as a coherent whole. In IIT, it is the intrinsic cause-effect power of the physical substrate, which doesn’t depend on what the system represents (Albantakis et al., 2023). HTCC also differs from global workspace theory (Dehaene & Changeux, 2011): in HTCC, global availability explains access and report, not the presence of experience itself.
5. Evolution #
HTCC proposes a scenario for how cognition evolved from simple homeostatic mechanisms to complex mental phenomena. This section traces that path, first for homeostatic regulation in general, and then for cognitive HVars. The examples illustrate each stage. They come from different lineages, and don’t by themselves establish the sequence.
5.1 From simple homeostasis to complex cognition #
- Primordial homeostasis. The story begins with simple homeostatic mechanisms in unicellular organisms, which kept essential variables within life-sustaining ranges. These are the basis for all later cognitive development (Damasio & Carvalho, 2013). Example: bacterial chemotaxis, where single cells move towards or away from chemical stimuli to maintain good conditions (Wadhams & Armitage, 2004).
- Multicellular coordination. As organisms became more complex, signaling between cells evolved, which allowed coordinated homeostatic responses across tissues and organs (Keijzer et al., 2013). Example: the endocrine system, which regulates many physiological processes through hormones (Hartenstein, 2006).
- Neural regulation. Nervous systems gave a faster, more flexible way to maintain homeostasis, and allowed more complex behavioral responses to the environment (Striedter, 2005). Example: the vertebrate hypothalamus, which regulates body temperature, hunger and thirst (Saper & Lowell, 2014).
- Predictive homeostasis. As neural systems became more sophisticated, they began to anticipate future states and prepare homeostatic responses in advance, i.e. allostasis (Section 2.1; Sterling, 2012). Example: the stress response, which prepares the body for anticipated challenges (McEwen & Wingfield, 2003).
- Cognitive maps and mental simulation. Internal models, or “cognitive maps”, of the environment were a major step in cognitive evolution. They let organisms simulate possible outcomes, which set the stage for cognitive HVars (Section 5.2) that pursue those outcomes as goals (Tolman, 1948). Example: spatial navigation in rats (O’Keefe & Nadel, 1978).
5.2 The emergence of cognitive HVars #
HTCC proposes that cognitive HVars mark the transition from basic physiological regulation to complex cognitive processes:
- Proto-cognitive HVars. The first cognitive HVars may have emerged as extensions of physiological regulation. They represented more abstract states that influenced survival and reproduction indirectly (Panksepp, 2005). Example: sensitization after injury, where an organism learns to protect an injured part of its body (Walters, 1994).
- Abstract goals. Representing and pursuing abstract goals was a major advance, because it allowed more flexible and adaptive behavior (Suddendorf & Corballis, 2007). Example: tool use in corvids (Emery & Clayton, 2004).
- Social HVars. As animals evolved complex social behavior, cognitive HVars emerged that regulate social interactions and hierarchies (Dunbar, 1998). Example: tracking social status in primates, which affects access to resources and health (Sapolsky, 2005).
- Metacognitive HVars. Metacognition, i.e. the ability to monitor and control one’s own cognitive processes, is a higher level of cognitive HVar (Metcalfe & Shimamura, 1994). Example: metamemory in primates, where animals show awareness of their own memory states (Hampton, 2001).
- Cultural and symbolic HVars. In humans, the ability to create and manipulate symbols led to cultural cognitive HVars, which greatly expanded the scope of homeostatic regulation (Deacon, 1997). Example: language, which allows the regulation of complex social and cultural states (Tomasello, 1999).
- Technological extension. Technology has extended the reach of cognitive HVars further, to the regulation of states far beyond immediate personal experience (Clark, 2003). Example: scientific instruments, which let cognitive HVars target quantities far beyond direct perception, from subatomic particles to distant galaxies (Humphreys, 2004).
HTCC proposes that this path, from simple homeostatic mechanisms to complex cognitive HVars, would account for the continuity between life and mind, and for the qualitative leaps in cognitive ability across species. On HTCC’s view, feelings are as old as homeostasis itself. Qualia came later, with the first self model (Section 4.4). Their richness would then have grown gradually, as self models became more integrated and precise. Where on this path the first self model appears is an open question (Section 10).
6. Philosophical implications #
HTCC offers new perspectives on three long-standing philosophical problems: the hard problem of consciousness, free will and determinism, and the nature of the self.
6.1 The hard problem of consciousness #
The hard problem, as Chalmers formulated it, asks why and how physical processes in the brain give rise to subjective experience (Chalmers, 1995).
- Reframing the question. Because qualia are implementation states of the self model (Section 4.3), the question shifts from “Why do we have subjective experiences?” to “How does the self model implement itself in different states?” (Seth, 2016).
- The explanatory gap. HTCC offers a candidate bridge between physical processes and subjective experience: the qualitative feel of experience is the state of the self model, which reflects the feelings of the underlying homeostatic system (Damasio, 2010). This relocates the explanatory gap more than it closes it. Why these states seem felt is still open (Section 10).
- Gradations of consciousness. Whether a system has experience depends on two conditions, but how rich that experience is varies with the integration and precision of the self model (Section 4.4). So the richness of experience grew gradually in evolution, not all at once (Section 5.2; Godfrey-Smith, 2020).
6.2 Free will and determinism #
- Two kinds of control. In HTCC, actions result from homeostatic processes that are caused by prior states, plus neural noise (Section 3.7), not by a separate act of choosing. HTCC distinguishes two kinds of control. Immediate actions follow the current landscape, moment to moment. Instantiating and configuring cognitive HVars reshapes the landscape itself, on slower timescales, and is where reflection, learning and planning act (Dennett, 2003).
- Levels of control. Splitting the slower kind by timescale gives three levels of control over behavior (Baumeister, 2008):
- No direct control over immediate actions.
- Indirect control, through instantiating and configuring cognitive HVars.
- Long-term control, through shaping the set of cognitive HVars over time.
- A compatibilist view. HTCC fits compatibilist accounts of free will, where actions can be both caused by prior events and free in a meaningful sense (Fischer & Ravizza, 1998). We don’t control our actions directly. But we can keep observing and adjusting our cognitive HVars, which in turn shape our actions, so that we end up taking the actions we wanted to take. The distinction between the levels is functional, not causal: configuring HVars is caused by prior states too. HTCC’s remaining commitment is that this functional capacity is the kind of freedom that matters (Section 10).
6.3 The nature of the self #
HTCC challenges the traditional idea of a unitary, persistent self.
- The self as a process. Because the self model is a dynamic process (Section 4.2), the self is a process, not a substance. This is in line with Buddhist views, and some contemporary Western views, of the self (Varela et al., 2016; Siderits et al., 2010).
- A multifaceted self. The HVars that the self model represents can pull in different directions. This may explain the sometimes conflicting sides of our personalities and behavior (Kurzban, 2010).
- The illusion of unity. The self model includes the sense of presence and agency (Section 4.1), which implies a single actor. The integration in the self model is real, but the single actor it implies is not (Metzinger, 2003).
- The extended self. The framework allows a self that includes not only the body and brain, but also the environment that the organism maintains homeostasis with. This resonates with theories of extended and embodied cognition (Clark & Chalmers, 1998).
By grounding consciousness, free will and the self in homeostatic processes, HTCC gives a naturalistic account of them that keeps much of their phenomenological richness, and opens these philosophical questions to empirical study.
7. Relation to other theories #
HTCC shares a lot with several contemporary theories, and adds its own perspective. This section summarizes how HTCC relates to them.
- Predictive processing and active inference (Clark, 2013; Friston, 2010; Hohwy, 2013). HTCC uses predictive loops to build the self model, which represents the system and its HVars, and proposes that qualia arise when the self model reflects the feelings of the underlying homeostatic system (Section 4). Related homeostatic and allostatic accounts of active inference include Pezzulo et al. (2015), Seth (2015) and Corcoran et al. (2020).
- Global workspace theory and integrated information theory (Baars, 1988; Tononi, 2008; Oizumi et al., 2014; Tononi & Koch, 2015; Tononi et al., 2016). HTCC shares IIT’s view that consciousness comes in degrees, but grades it by the integration of the self model, not by IIT’s intrinsic integration (Section 4.4). It gives global availability a narrower role than GWT does: availability explains access and report, not the presence of experience (Section 4.4). HTCC also proposes how consciousness connects to homeostatic regulation, which these theories leave open (Section 1.2).
- Feelings and the evolution of mind (Damasio, 2010; Damasio & Carvalho, 2013; Godfrey-Smith, 2016, 2020). HTCC shares the view that mind and the self are rooted in homeostatic regulation, and that mind evolved continuously from life (Section 5).
- Control theory and homeostatic reinforcement learning (Powers, 1973; Keramati & Gutkin, 2014). HVars and the homeostatic landscape (Section 3) build on both, and extend them from physiological variables to variables that the organism instantiates for itself (Section 2.3).
- Embodied, enactive and extended cognition (Varela et al., 2016; Thompson, 2007; Chemero, 2011; O’Regan & Noë, 2001; Kiverstein & Miller, 2015; Wilson & Foglia, 2017). HTCC shares the enactive view that an organism’s stakes come from its self-maintenance (Weber & Varela, 2002; Di Paolo, 2005). Man and Damasio (2019) apply the same view to machines: a machine would need a body whose homeostasis it has to maintain before it could have feelings. HTCC agrees, and adds a self model as the further condition for qualia (Section 4.4). HTCC’s self is a process, not a substance, and can extend into the environment that the organism maintains homeostasis with (Section 6.3).
8. Applications #
If HTCC is right, it suggests applications in three areas. These are directions, not worked-out methods.
- Psychiatry and neurology. Some mental disorders might be described as problems in the life cycle of cognitive HVars, i.e. in creating, configuring, retiring or reactivating them (Pezzulo et al., 2019). Conditions such as anosognosia and phantom limbs might be described as mismatches between the self model and the body it represents (Ramachandran & Hirstein, 1998). Disorders of consciousness might be assessed through the integrity of the self model (Gosseries et al., 2014).
- Artificial intelligence. Agents built from physiological and cognitive HVars may be more robust and adaptable (Vernon et al., 2015; Kelkar, 2021).
- Artificial consciousness. HTCC implies that a self model alone isn’t enough for an artificial system to be conscious. It also needs an underlying homeostatic system, which gives it stakes, and feelings relative to them, for the self model to reflect (Section 4.4). HTCC doesn’t rule out software. What matters is how the system is built. A typical robot’s battery and temperature management is a task its designers assigned, carried out by parts the robot doesn’t maintain, so nothing is at stake for the robot in the sense of Section 4.3. And if the robot has a self model, the model typically reads the battery level as data, rather than being implemented as loops that include the battery’s regulation (Section 4.2). Such a robot has neither feelings in HTCC’s sense nor a self model that could reflect them. An artificial system with stakes of its own, and a self model implemented as loops that include their regulation, would be conscious on HTCC’s view. The open criteria for both conditions (Section 10) therefore matter for research on artificial consciousness (Reggia et al., 2020).
9. Testable predictions and research methods #
9.1 Predictions #
These predictions are broad. Section 10 discusses the need for sharper ones.
- State-dependent trade-offs. If cognitive and physiological HVars compete in one landscape (Section 3.3), the rate at which a person trades a cognitive goal against a physiological need should change with physiological state. Finding no such dependence would count against HTCC. Homeostatic reinforcement learning shares this expectation (Keramati & Gutkin, 2014), so confirming it would support HTCC without distinguishing it. A test that distinguishes them needs the formal model in Section 10, including the shape of the landscape.
- Neural signatures of HVars. If a cognitive HVar has its own estimate and target (Section 2.3), changing only the target, with the stimuli and the required actions held fixed, should change neural activity that tracks the deviation from the target. Activity that reflects sensory processing or motor preparation shouldn’t change in the same way (Critchley & Harrison, 2013).
- Hierarchical organization. Brain activity should reflect a hierarchy of homeostatic processes (Kiebel et al., 2008; Badcock et al., 2019).
- Cognitive–physiological interactions. Changes in cognitive HVars should affect physiological HVars, and the other way around (Thayer & Lane, 2000).
- Dimensions of consciousness. Differences between global states of consciousness, such as sleep, anaesthesia and disorders of consciousness, should track whether the self model is running, and how integrated and precise it is (Section 4.4; Bayne et al., 2016).
9.2 A first experiment: breath holding #
Breath holding lets the cognitive target, the physiological state and attention be manipulated separately.
- Manipulation. Participants hold their breath with different instructed targets, e.g. 30 seconds, 60 seconds, or as long as they can. Goal strength is manipulated separately from the target, e.g. by the reward for reaching it. In some holds, the target is raised partway through. Physiological state is set before each hold, e.g. by breathing air or oxygen first, which lengthens holds (Parkes, 2006). Attention is manipulated separately, by asking participants to count or to attend to the urge to breathe.
- Observations. Behavioral: when the hold ends. Physiological: end-tidal carbon dioxide and blood oxygen saturation at the breakpoint. Subjective: separate ratings, during and after the hold, of the wanting to breathe, the determination to complete the hold, and how each passing second feels along each goal. Section 4.3 predicts that the seconds feel good along the hold and bad along breathing at the same time. Comparing the ratings with the other measures tests these mappings separately from the regulatory claims.
- Two ways a hold ends. A hold is target-limited if it ends at the target, and physiologically limited if it ends at a breakpoint before the target (Figure 3). The analysis keeps the two apart.
- What HTCC predicts. The study tests whether the strength of the goal trades off against physiology. Among physiologically limited holds from matched starting states, a stronger goal should delay the breakpoint and push it to worse blood gases. A worse starting physiological state should turn more holds from target-limited into physiologically limited. Whether a longer target also strengthens the goal is a separate assumption. If the goal’s pull doesn’t depend on the target, as Figure 3 draws it, holds with different targets break at the same point once physiology wins. Raising the target partway through a hold reconfigures the active HVar (Section 2.3), and should extend holds that would otherwise have ended at the old target.
- What would challenge HTCC. Suppose participants adopt the targets and respond to the rewards, which target-limited stopping and the choice of rewards in the easier conditions can confirm. If, among physiologically limited holds from matched states, a stronger goal doesn’t delay the breakpoint, the competition proposed in Section 3.3 fails for this task. A breakpoint that doesn’t change with the target challenges only the added assumption that longer targets strengthen the goal. A physiological limit that dominates every condition would make the result uninformative, not negative, so the conditions should include holds that physiology allows and holds that it doesn’t.
- Alternatives. Homeostatic reinforcement learning and other accounts of goal-directed control also predict that targets change behavior (Keramati & Gutkin, 2014). So the design constrains HTCC without singling it out. Separating the models needs the formal model in Section 10, tested in a preregistered comparison of divergent predictions, like the one that tested two theories of consciousness against each other (Cogitate Consortium et al., 2025).
9.3 Experimental paradigms #
- Neuroimaging. Use fMRI or EEG to identify the neural correlates of different HVars and their interactions (Seth & Friston, 2016).
- Behavioral experiments. Design tasks that manipulate cognitive HVars, and measure the effects on physiology and behavior (Barrett & Simmons, 2015).
- Clinical studies. Investigate how disruptions to specific HVars relate to the symptoms of psychiatric and neurological disorders (Paulus & Stein, 2006).
- Comparative studies. Compare homeostatic processes across species to test HTCC’s evolutionary predictions (Godfrey-Smith, 2020).
- Integration mechanisms. Study the mechanisms that integrate the aspects of the system, and its HVars, into one self model, which may shed light on the binding problem (Tononi & Koch, 2015).
9.4 Computational modeling #
Computational models will be key to developing and testing HTCC:
- Agent-based models. Simulate agents with homeostatic architectures, such as the Cognitive Homeostatic Agent outlined in Kelkar (2021), and study the cognitive behaviors that emerge (Friston et al., 2015).
- Neural network models. Implement HTCC principles in artificial neural networks, and study how they process and integrate information (Kriegeskorte & Douglas, 2018).
- Dynamical systems models. Use dynamical systems theory to model how multiple HVars interact (Rabinovich et al., 2015).
10. Open challenges and future work #
This paper states HTCC at the level of principles. Several challenges remain before it is a complete, testable theory. Items 1 to 5 concern HTCC’s foundations, and affect how its claims should be read. Items 6 to 10 extend the theory. We will address them in subsequent papers.
- A formal model. Section 3.1 states what a formal model of the landscape has to preserve. The model also has to say how the contributions of different HVars are scaled against each other, and what
tracks. Neuroeconomics has studied how the brain might encode a common scale (Levy & Glimcher, 2012), and the dissociation between wanting and liking shows that motivation and pleasure can come apart (Berridge & Robinson, 2016). The model should produce quantitative predictions, building on control theory (Powers, 1973) and homeostatic reinforcement learning (Keramati & Gutkin, 2014). - Falsifiability. If any behavior can be redescribed as the regulation of some HVar, the conjecture that all cognition is homeostatic forbids nothing. The criterion in Section 2.3 restricts what counts as an HVar, and Section 9.2 describes an experiment whose outcomes could challenge one of its predictions. HTCC still needs predictions that distinguish it from other homeostatic models, in quantitative form.
- The mechanism of the life cycle. Section 2.3 describes the life cycle of a cognitive HVar, but not the mechanism that creates an HVar, or that decides whether it persists, goes dormant or is retired. Many goals are reached once and not maintained, which fits poorly with the defended ranges of classic homeostasis.
- From feelings to qualia. Section 4.3 states what it means for the self model to reflect a feeling, and proposes how the intensity, valence and affective character of feelings follow from each HVar’s state and its changes. These mappings are provisional, and the account of perceptual content is less developed than the account of affect. HTCC also doesn’t yet explain why the self model’s states seem felt, rather than being dynamics with no experience. One candidate position is illusionism (Frankish, 2016), which has to answer the objection that if there is no phenomenal fact, nothing explains why pain is bad (Kammerer, 2019).
- Which systems have stakes and a self model. A thermostat regulates a room’s temperature, but not its own continued existence, and a candle flame maintains itself but doesn’t regulate anything. Section 8 argues that typical robots have no stakes, and that a self model that reads their state as data doesn’t reflect feelings. HTCC needs principled criteria for both, including how integrated a model of oneself has to be, when a self model is implemented as loops that include the regulation of HVars, rather than reading them as data (Section 4.2), and what makes regulation the system’s own rather than an assigned task (Section 4.3). Sections 4.2, 4.3 and 8 state HTCC’s provisional criteria, which need to be made precise. Together, these criteria decide which systems are conscious (Section 4.4).
- Attention. Section 3.2 treats attention as a modulator of the homeostatic landscape, but doesn’t say what controls it. Whether attention is itself regulated by HVars needs to be worked out.
- Agency. Section 6.2 distinguishes immediate action from configuring cognitive HVars as kinds of control, not as processes with different causal status. Whether that functional distinction is enough for the freedom people care about is a philosophical commitment that needs defending.
- Language. Section 5.2 gives only a brief account of language. A full account of language as cognitive homeostasis remains to be developed.
- Comparison with active inference and enactivism. Section 1.3 states what HTCC adds to Kelkar (2021) and Pezzulo et al. (2015). A detailed comparison with active inference, which already unifies physiological regulation and behavior under one formal principle (Friston, 2010), and with enactivism (Weber & Varela, 2002; Di Paolo, 2005; Thompson, 2007), remains to be done.
- Empirical tests. The predictions in Section 9.1 need concrete experimental designs beyond the one in Section 9.2, and where possible, reanalysis of existing open datasets on how physiological state changes choices.
11. Conclusion #
HTCC proposes a unified framework for understanding mind and brain. It grounds cognition in the basic biological principle of homeostasis, and proposes one account of a wide range of mental phenomena, from goal setting to complex reasoning and consciousness.
HTCC connects several levels of explanation, from evolutionary biology to neuroscience and philosophy of mind. It offers new perspectives on long-standing questions such as the hard problem of consciousness, the nature of the self and free will. It also suggests new approaches to understanding and treating mental disorders, and to building more sophisticated AI systems.
Many questions remain open (Section 10), but HTCC gives a theoretical framework from which testable predictions can be derived (Section 9.1), and it opens new directions for empirical research.
References #
- Adolphs, R. (2015). The unsolved problems of neuroscience. Trends in Cognitive Sciences, 19(4), 173–175.
- Albantakis, L., Barbosa, L., Findlay, G., Grasso, M., Haun, A. M., Marshall, W., Mayner, W. G. P., Zaeemzadeh, A., Boly, M., Juel, B. E., Sasai, S., Fujii, K., David, I., Hendren, J., Lang, J. P., & Tononi, G. (2023). Integrated information theory (IIT) 4.0: Formulating the properties of phenomenal existence in physical terms. PLoS Computational Biology, 19(10), e1011465.
- Ashby, W. R. (1952). Design for a brain. Chapman & Hall.
- Baars, B. J. (1988). A cognitive theory of consciousness. Cambridge University Press.
- Baars, B. J. (2005). Global workspace theory of consciousness: toward a cognitive neuroscience of human experience. Progress in Brain Research, 150, 45–53.
- Badcock, P. B., Friston, K. J., & Ramstead, M. J. (2019). The hierarchically mechanistic mind: A free-energy formulation of the human psyche. Physics of Life Reviews, 31, 104–121.
- Barrett, L. F., & Simmons, W. K. (2015). Interoceptive predictions in the brain. Nature Reviews Neuroscience, 16(7), 419–429.
- Baumeister, R. F. (2008). Free will in scientific psychology. Perspectives on Psychological Science, 3(1), 14–19.
- Bayne, T., Hohwy, J., & Owen, A. M. (2016). Are there levels of consciousness? Trends in Cognitive Sciences, 20(6), 405–413.
- Beaty, R. E., Benedek, M., Wilkins, R. W., Jauk, E., Fink, A., Silvia, P. J., … & Neubauer, A. C. (2014). Creativity and the default network: A functional connectivity analysis of the creative brain at rest. Neuropsychologia, 64, 92–98.
- Berridge, K. C., & Robinson, T. E. (2016). Liking, wanting, and the incentive-sensitization theory of addiction. American Psychologist, 71(8), 670–679.
- Blanke, O., Slater, M., & Serino, A. (2015). Behavioral, neural, and computational principles of bodily self-consciousness. Neuron, 88(1), 145–166.
- Breakspear, M. (2017). Dynamic models of large-scale brain activity. Nature Neuroscience, 20(3), 340–352.
- Cannon, W. B. (1929). Organization for physiological homeostasis. Physiological Reviews, 9(3), 399–431.
- Carrasco, M. (2011). Visual attention: The past 25 years. Vision Research, 51(13), 1484–1525.
- Carver, C. S., & Scheier, M. F. (1982). Control theory: A useful conceptual framework for personality–social, clinical, and health psychology. Psychological Bulletin, 92(1), 111–135.
- Chalmers, D. J. (1995). Facing up to the problem of consciousness. Journal of Consciousness Studies, 2(3), 200–219.
- Chemero, A. (2011). Radical embodied cognitive science. MIT Press.
- Christoff, K., Irving, Z. C., Fox, K. C., Spreng, R. N., & Andrews-Hanna, J. R. (2016). Mind-wandering as spontaneous thought: a dynamic framework. Nature Reviews Neuroscience, 17(11), 718–731.
- Cisek, P., & Kalaska, J. F. (2010). Neural mechanisms for interacting with a world full of action choices. Annual Review of Neuroscience, 33, 269–298.
- Clark, A. (2003). Natural-born cyborgs: Minds, technologies, and the future of human intelligence. Oxford University Press.
- Clark, A. (2013). Whatever next? Predictive brains, situated agents, and the future of cognitive science. Behavioral and Brain Sciences, 36(3), 181–204.
- Clark, A., & Chalmers, D. (1998). The extended mind. Analysis, 58(1), 7–19.
- Conant, R. C., & Ashby, W. R. (1970). Every good regulator of a system must be a model of that system. International Journal of Systems Science, 1(2), 89–97.
- Corcoran, A. W., Pezzulo, G., & Hohwy, J. (2020). From allostatic agents to counterfactual cognisers: active inference, biological regulation, and the origins of cognition. Biology & Philosophy, 35(3), 1–45.
- Cogitate Consortium, Ferrante, O., Gorska-Klimowska, U., Henin, S., Hirschhorn, R., Khalaf, A., Lepauvre, A., Liu, L., Richter, D., Vidal, Y., Bonacchi, N., Brown, T., Sripad, P., Armendariz, M., Bendtz, K., Ghafari, T., Hetenyi, D., Jeschke, J., Kozma, C., … Melloni, L. (2025). Adversarial testing of global neuronal workspace and integrated information theories of consciousness. Nature, 642(8066), 133–142.
- Craig, A. D. (2009). How do you feel—now? The anterior insula and human awareness. Nature Reviews Neuroscience, 10(1), 59–70.
- Critchley, H. D., & Harrison, N. A. (2013). Visceral influences on brain and behavior. Neuron, 77(4), 624–638.
- Dai, H., Milkman, K. L., & Riis, J. (2014). The fresh start effect: Temporal landmarks motivate aspirational behavior. Management Science, 60(10), 2563–2582.
- Damasio, A. (2010). Self comes to mind: Constructing the conscious brain. Pantheon/Random House.
- Damasio, A., & Carvalho, G. B. (2013). The nature of feelings: evolutionary and neurobiological origins. Nature Reviews Neuroscience, 14(2), 143–152.
- Dampney, R. A., et al. (2002). Central mechanisms underlying short- and long-term regulation of the cardiovascular system. Clinical and Experimental Pharmacology and Physiology, 29(4), 261–268.
- Deacon, T. W. (1997). The symbolic species: The co-evolution of language and the brain. W. W. Norton & Company.
- Dehaene, S., & Changeux, J. P. (2011). Experimental and theoretical approaches to conscious processing. Neuron, 70(2), 200–227.
- Dehaene, S., Lau, H., & Kouider, S. (2017). What is consciousness, and could machines have it? Science, 358(6362), 486–492.
- Dennett, D. C. (1988). Quining qualia. In A. Marcel & E. Bisiach (Eds.), Consciousness in contemporary science. Oxford University Press.
- Dennett, D. C. (2003). Freedom evolves. Viking.
- Di Paolo, E. A. (2005). Autopoiesis, adaptivity, teleology, agency. Phenomenology and the Cognitive Sciences, 4(4), 429–452.
- Diamond, A. (2013). Executive functions. Annual Review of Psychology, 64, 135–168.
- Dunbar, R. I. M. (1998). The social brain hypothesis. Evolutionary Anthropology: Issues, News, and Reviews, 6(5), 178–190.
- Edelman, G. M., & Tononi, G. (2000). A universe of consciousness: How matter becomes imagination. Basic Books.
- Emery, N. J., & Clayton, N. S. (2004). The mentality of crows: convergent evolution of intelligence in corvids and apes. Science, 306(5703), 1903–1907.
- Felleman, D. J., & Van Essen, D. C. (1991). Distributed hierarchical processing in the primate cerebral cortex. Cerebral Cortex, 1(1), 1–47.
- Fischer, J. M., & Ravizza, M. (1998). Responsibility and control: A theory of moral responsibility. Cambridge University Press.
- Fleming, S. M., & Dolan, R. J. (2012). The neural basis of metacognitive ability. Philosophical Transactions of the Royal Society B: Biological Sciences, 367(1594), 1338–1349.
- Frankish, K. (2016). Illusionism as a theory of consciousness. Journal of Consciousness Studies, 23(11–12), 11–39.
- Friston, K. (2010). The free-energy principle: a unified brain theory? Nature Reviews Neuroscience, 11(2), 127–138.
- Friston, K. (2012). The history of the future of the Bayesian brain. NeuroImage, 62(2), 1230–1233.
- Friston, K., Rigoli, F., Ognibene, D., Mathys, C., Fitzgerald, T., & Pezzulo, G. (2015). Active inference and epistemic value. Cognitive Neuroscience, 6(4), 187–214.
- Fukushima, K. (1980). Neocognitron: A self-organizing neural network model for a mechanism of pattern recognition unaffected by shift in position. Biological Cybernetics, 36(4), 193–202.
- Georgopoulos, A. P., Schwartz, A. B., & Kettner, R. E. (1986). Neuronal population coding of movement direction. Science, 233(4771), 1416–1419.
- Godfrey-Smith, P. (2016). Other minds: The octopus, the sea, and the deep origins of consciousness. Farrar, Straus and Giroux.
- Godfrey-Smith, P. (2020). Metazoa: Animal life and the birth of the mind. Farrar, Straus and Giroux.
- Gosseries, O., Di, H., Laureys, S., & Boly, M. (2014). Measuring consciousness in severely damaged brains. Annual Review of Neuroscience, 37, 457–478.
- Haggard, P. (2017). Sense of agency in the human brain. Nature Reviews Neuroscience, 18(4), 196–207.
- Hampton, R. R. (2001). Rhesus monkeys know when they remember. Proceedings of the National Academy of Sciences, 98(9), 5359–5362.
- Hartenstein, V. (2006). The neuroendocrine system of invertebrates: a developmental and evolutionary perspective. Journal of Endocrinology, 190(3), 555–570.
- Hawkins, J., Ahmad, S., & Cui, Y. (2017). A theory of how columns in the neocortex enable learning the structure of the world. Frontiers in Neural Circuits, 11, 81.
- Hawkins, J., & Blakeslee, S. (2004). On intelligence. Times Books.
- Hofstadter, D. R. (1979). Gödel, Escher, Bach: An eternal golden braid. Basic Books.
- Hohwy, J. (2013). The predictive mind. Oxford University Press.
- Hopfield, J. J. (1982). Neural networks and physical systems with emergent collective computational abilities. Proceedings of the National Academy of Sciences, 79(8), 2554–2558.
- Hubel, D. H., & Wiesel, T. N. (1962). Receptive fields, binocular interaction and functional architecture in the cat’s visual cortex. The Journal of Physiology, 160(1), 106–154.
- Humphreys, P. (2004). Extending ourselves: Computational science, empiricism, and scientific method. Oxford University Press.
- Jacob, F. (1977). Evolution and tinkering. Science, 196(4295), 1161–1166.
- Kammerer, F. (2019). The normative challenge for illusionist views of consciousness. Ergo, 6(32).
- Keijzer, F., Van Duijn, M., & Lyon, P. (2013). What nervous systems do: early evolution, input–output, and the skin brain thesis. Adaptive Behavior, 21(2), 67–85.
- Kelkar, A. (2018). Homeostasis theory of consciousness: Solving the hard problem using physiological correlates of consciousness. Poster presented at the 22nd annual meeting of the Association for the Scientific Study of Consciousness (ASSC 22), Kraków, Poland. doi:10.13140/RG.2.2.35033.83047.
- Kelkar, A. (2021). Cognitive homeostatic agents. In Proceedings of the 20th International Conference on Autonomous Agents and Multiagent Systems (AAMAS 2021), Blue Sky Ideas track. IFAAMAS. arXiv:2103.03359.
- Keramati, M., & Gutkin, B. (2014). Homeostatic reinforcement learning for integrating reward collection and physiological stability. eLife, 3, e04811.
- Kiebel, S. J., Daunizeau, J., & Friston, K. J. (2008). A hierarchy of time-scales and the brain. PLoS Computational Biology, 4(11), e1000209.
- Kiverstein, J., & Miller, M. (2015). The embodied brain: towards a radical embodied cognitive neuroscience. Frontiers in Human Neuroscience, 9, 237.
- Kriegeskorte, N., & Douglas, P. K. (2018). Cognitive computational neuroscience. Nature Neuroscience, 21(9), 1148–1160.
- Kurzban, R. (2010). Why everyone (else) is a hypocrite: Evolution and the modular mind. Princeton University Press.
- Lau, H., & Rosenthal, D. (2011). Empirical support for higher-order theories of conscious awareness. Trends in Cognitive Sciences, 15(8), 365–373.
- Levy, D. J., & Glimcher, P. W. (2012). The root of all value: a neural common currency for choice. Current Opinion in Neurobiology, 22(6), 1027–1038.
- Man, K., & Damasio, A. (2019). Homeostasis and soft robotics in the design of feeling machines. Nature Machine Intelligence, 1(10), 446–452.
- Maturana, H. R., & Varela, F. J. (1980). Autopoiesis and cognition: The realization of the living. D. Reidel.
- McEwen, B. S., & Wingfield, J. C. (2003). The concept of allostasis in biology and biomedicine. Hormones and Behavior, 43(1), 2–15.
- Melzack, R., & Wall, P. D. (1965). Pain mechanisms: a new theory. Science, 150(3699), 971–979.
- Metcalfe, J., & Shimamura, A. P. (Eds.). (1994). Metacognition: Knowing about knowing. MIT Press.
- Metzinger, T. (2003). Being no one: The self-model theory of subjectivity. MIT Press.
- Miller, E. K., & Cohen, J. D. (2001). An integrative theory of prefrontal cortex function. Annual Review of Neuroscience, 24(1), 167–202.
- Mischel, W., Shoda, Y., & Rodriguez, M. I. (1989). Delay of gratification in children. Science, 244(4907), 933–938.
- Modell, H., et al. (2015). A physiologist’s view of homeostasis. Advances in Physiology Education, 39(4), 259–266.
- Moore-Ede, M. C. (1986). Physiology of the circadian timing system: predictive versus reactive homeostasis. American Journal of Physiology-Regulatory, Integrative and Comparative Physiology, 250(5), R737–R752.
- Morrison, S. F., & Nakamura, K. (2019). Central mechanisms for thermoregulation. Annual Review of Physiology, 81, 285–308.
- Mrosovsky, N. (1990). Rheostasis: The physiology of change. Oxford University Press.
- Newell, A., & Simon, H. A. (1972). Human problem solving. Prentice-Hall.
- O’Keefe, J., & Nadel, L. (1978). The hippocampus as a cognitive map. Clarendon Press.
- O’Regan, J. K., & Noë, A. (2001). A sensorimotor account of vision and visual consciousness. Behavioral and Brain Sciences, 24(5), 939–973.
- Oizumi, M., Albantakis, L., & Tononi, G. (2014). From the phenomenology to the mechanisms of consciousness: integrated information theory 3.0. PLoS Computational Biology, 10(5), e1003588.
- Panksepp, J. (2005). Affective consciousness: Core emotional feelings in animals and humans. Consciousness and Cognition, 14(1), 30–80.
- Parkes, M. J. (2006). Breath-holding and its breakpoint. Experimental Physiology, 91(1), 1–15.
- Paulus, M. P., & Stein, M. B. (2006). An insular view of anxiety. Biological Psychiatry, 60(4), 383–387.
- Pezzulo, G., Maisto, D., Barca, L., & Van den Bergh, O. (2019). Symptom perception from a predictive processing perspective. Clinical Psychology in Europe, 1(4), 1–14.
- Pezzulo, G., Rigoli, F., & Friston, K. (2015). Active Inference, homeostatic regulation and adaptive behavioural control. Progress in Neurobiology, 134, 17–35.
- Posner, M. I., & Rothbart, M. K. (2007). Research on attention networks as a model for the integration of psychological science. Annual Review of Psychology, 58, 1–23.
- Pouget, A., Dayan, P., & Zemel, R. (2000). Information processing with population codes. Nature Reviews Neuroscience, 1(2), 125–132.
- Powers, W. T. (1973). Behavior: The control of perception. Aldine.
- Rabinovich, M. I., Simmons, A. N., & Varona, P. (2015). Dynamical bridge between brain and mind. Trends in Cognitive Sciences, 19(8), 453–461.
- Ramachandran, V. S., & Hirstein, W. (1998). The perception of phantom limbs. Brain, 121(9), 1603–1630.
- Rao, R. P. N., & Ballard, D. H. (1999). Predictive coding in the visual cortex: a functional interpretation of some extra-classical receptive-field effects. Nature Neuroscience, 2(1), 79–87.
- Reggia, J. A., Katz, G. E., & Davis, G. P. (2020). Artificial conscious intelligence. Journal of Artificial Intelligence and Consciousness, 7(01), 95–107.
- Riesenhuber, M., & Poggio, T. (1999). Hierarchical models of object recognition in cortex. Nature Neuroscience, 2(11), 1019–1025.
- Saper, C. B., & Lowell, B. B. (2014). The hypothalamus. Current Biology, 24(23), R1111–R1116.
- Sapolsky, R. M. (2005). The influence of social hierarchy on primate health. Science, 308(5722), 648–652.
- Schultz, W., Dayan, P., & Montague, P. R. (1997). A neural substrate of prediction and reward. Science, 275(5306), 1593–1599.
- Seth, A. K. (2013). Interoceptive inference, emotion, and the embodied self. Trends in Cognitive Sciences, 17(11), 565–573.
- Seth, A. K. (2015). The cybernetic Bayesian brain. In Open MIND. MIND Group.
- Seth, A. K. (2016). The real problem. Aeon. https://aeon.co/essays/the-hard-problem-of-consciousness-is-a-distraction-from-the-real-one
- Seth, A. K., & Friston, K. J. (2016). Active interoceptive inference and the emotional brain. Philosophical Transactions of the Royal Society B: Biological Sciences, 371(1708), 20160007.
- Seth, A. K., Suzuki, K., & Critchley, H. D. (2012). An interoceptive predictive coding model of conscious presence. Frontiers in Psychology, 2, 395.
- Siderits, M., Thompson, E., & Zahavi, D. (Eds.). (2010). Self, no self? Perspectives from analytical, phenomenological, and Indian traditions. Oxford University Press.
- Steel, P., & König, C. J. (2006). Integrating theories of motivation. Academy of Management Review, 31(4), 889–913.
- Sterling, P. (2012). Allostasis: a model of predictive regulation. Physiology & Behavior, 106(1), 5–15.
- Sterling, P., & Eyer, J. (1988). Allostasis: A new paradigm to explain arousal pathology. In S. Fisher & J. Reason (Eds.), Handbook of Life Stress, Cognition and Health (pp. 629–649). John Wiley & Sons.
- Striedter, G. F. (2005). Principles of brain evolution. Sinauer Associates.
- Suddendorf, T., & Corballis, M. C. (2007). The evolution of foresight: What is mental time travel, and is it unique to humans? Behavioral and Brain Sciences, 30(3), 299–313.
- Sutton, R. S., & Barto, A. G. (2018). Reinforcement learning: An introduction (2nd ed.). MIT Press.
- Synofzik, M., Vosgerau, G., & Newen, A. (2008). Beyond the comparator model: A multifactorial two-step account of agency. Consciousness and Cognition, 17(1), 219–239.
- Thayer, J. F., & Lane, R. D. (2000). A model of neurovisceral integration in emotion regulation and dysregulation. Journal of Affective Disorders, 61(3), 201–216.
- Thiele, A., & Bellgrove, M. A. (2018). Neuromodulation of attention. Neuron, 97(4), 769–785.
- Thompson, E. (2007). Mind in life: Biology, phenomenology, and the sciences of mind. Harvard University Press.
- Thompson, E., & Varela, F. J. (2001). Radical embodiment: neural dynamics and consciousness. Trends in Cognitive Sciences, 5(10), 418–425.
- Tolman, E. C. (1948). Cognitive maps in rats and men. Psychological Review, 55(4), 189–208.
- Tomasello, M. (1999). The cultural origins of human cognition. Harvard University Press.
- Tononi, G. (2008). Consciousness as integrated information: a provisional manifesto. The Biological Bulletin, 215(3), 216–242.
- Tononi, G., Boly, M., Massimini, M., & Koch, C. (2016). Integrated information theory: from consciousness to its physical substrate. Nature Reviews Neuroscience, 17(7), 450–461.
- Tononi, G., & Koch, C. (2015). Consciousness: here, there and everywhere? Philosophical Transactions of the Royal Society B: Biological Sciences, 370(1668), 20140167.
- Varela, F. J. (1999). Present-time consciousness. Journal of Consciousness Studies, 6(2–3), 111–140.
- Varela, F. J., Thompson, E., & Rosch, E. (2016). The embodied mind: Cognitive science and human experience. MIT Press.
- Vaswani, A., Shazeer, N., Parmar, N., Uszkoreit, J., Jones, L., Gomez, A. N., Kaiser, Ł., & Polosukhin, I. (2017). Attention is all you need. In Advances in Neural Information Processing Systems 30 (NeurIPS 2017). arXiv:1706.03762.
- Vernon, D., Lowe, R., Thill, S., & Ziemke, T. (2015). Embodied cognition and circular causality: on the role of constitutive autonomy in the reciprocal coupling of perception and action. Frontiers in Psychology, 6, 1660.
- Wadhams, G. H., & Armitage, J. P. (2004). Making sense of it all: bacterial chemotaxis. Nature Reviews Molecular Cell Biology, 5(12), 1024–1037.
- Walters, E. T. (1994). Injury-related behavior and neuronal plasticity: an evolutionary perspective on sensitization, hyperalgesia, and analgesia. International Review of Neurobiology, 36, 325–427.
- Weber, A., & Varela, F. J. (2002). Life after Kant: Natural purposes and the autopoietic foundations of biological individuality. Phenomenology and the Cognitive Sciences, 1, 97–125.
- Wiener, N. (1948). Cybernetics: Or control and communication in the animal and the machine. MIT Press.
- Wilson, R. A., & Foglia, L. (2017). Embodied cognition. In E. N. Zalta (Ed.), The Stanford Encyclopedia of Philosophy (Spring 2017 Edition).
- Windt, J. M., Nielsen, T., & Thompson, E. (2016). Does consciousness disappear in dreamless sleep? Trends in Cognitive Sciences, 20(12), 871–882.
- Wittmann, M. (2011). Moments in time. Frontiers in Integrative Neuroscience, 5, 66.
- Wolpert, D. M., & Ghahramani, Z. (2000). Computational principles of movement neuroscience. Nature Neuroscience, 3(11), 1212–1217.
- Wrosch, C., Scheier, M. F., Miller, G. E., Schulz, R., & Carver, C. S. (2003). Adaptive self-regulation of unattainable goals: Goal disengagement, goal reengagement, and subjective well-being. Personality and Social Psychology Bulletin, 29(12), 1494–1508.
Further reading #
- Bayne, T., & Chalmers, D. J. (2003). What is the unity of consciousness? In A. Cleeremans (Ed.), The Unity of Consciousness. Oxford University Press.
- Chalmers, D. J. (2013). Panpsychism and panprotopsychism. The Amherst Lecture in Philosophy, 8, 1–35.
- Henrich, J., Heine, S. J., & Norenzayan, A. (2010). The weirdest people in the world? Behavioral and Brain Sciences, 33(2–3), 61–83.
- Nahmias, E. (2014). Is free will an illusion? Confronting challenges from the modern mind sciences. Moral Psychology, 4, 1–25.
- Northoff, G., & Lamme, V. (2020). Neural signs and mechanisms of consciousness: Is there a potential convergence of theories of consciousness in sight? Neuroscience & Biobehavioral Reviews, 118, 568–587.
- Seth, A. K., Dienes, Z., Cleeremans, A., Overgaard, M., & Pessoa, L. (2008). Measuring consciousness: relating behavioural and neurophysiological approaches. Trends in Cognitive Sciences, 12(8), 314–321.
- Zelazo, P. D. (2015). Executive function: Reflection, iterative reprocessing, complexity, and the developing brain. Developmental Review, 38, 55–68.